Tuesday, July 26, 2022

A critical analysis of the Klamelisaurus paper by Moore et al. (2020)

In the 1980s, new eusauropod remains were unearthed in the Middle-Late Jurassic (Callovian-Oxfordian) Shishugou Formation of Xinjiang, and they would be eventually named Bellusaurus sui  Dong, 1990 and Klamelisaurus gobiensis Zhao, 1993, constituting the first eusauropod taxa to be described from Xinjiang since the description of Tienshanosaurus in 1937. Although Klamelisaurus is based on substantial postcranial remains like the vast majority of eusauropod taxa described from the Shaximiao Formation in Sichuan, and it was assigned to a new subfamily, Klamelisaurinae, within Brachiosauridae, its relationship to other Jurassic eusauropods from East Asia was clouded by an outdated diagnosis, the hypothesis about Klamelisaurus being an adult Bellusaurus, and the need for a comprehensive revision of the well-known genera Mamenchisaurus and Omeisaurus, and thus Upchurch et al. (2004) listed Klamelisaurus as Eusauropoda incertae sedis. Recently, Moore et al. (2020) published a redescription of Klamelisaurus based on comparisons with mamenchisaurid taxa, and cladistic analyses of this taxon found it to be a derived member of Mamenchisauridae as suggested by Upchurch et al. (2004), with some topologies recovering it as sister to Euhelopus, the type genus of Euhelopodidae. Given that some cladistic analyses by Moore et al (2020) create some implications for the validity of Euhelopodidae with respect to Mamenchisauridae considering the recovery of Euhelopus as a titanosauriform, I'll go into certain aspects of the paper by Moore et al. (2020) regarding Klamelisaurus, namely conclusions from results of phylogenetic analyses of this taxon.

Cast of the holotype postcranial skeleton of Klamelisaurus gobiensis on display at a museum in Japan, with a skull cast mounted at the front of the cervical region (courtesy of Wikimedia Commons)  

In the systematic paleontology section of their paper, Moore et al. carry out a comprehensive approach to distinguishing Klamelisaurus from other Jurassic eusauropods from East Asia. As correctly noted by the authors, nearly all the characters included by Zhao (1993) in his diagnosis of Klamelisaurus are virtually either plesiomorphic for non-neosauropod eusauropods or present in other mamenchisaurids, similar to the diagnoses given by Dong et al. (1983) for some eusauropod taxa from Sichuan, and among the characters listed by the authors in the revised diagnosis for Klamelisaurus gobiensis, the scabrous, sheet-like anterior extensions of the spinoprezygapophyseal laminae (SPRL) in the middle to posterior cervical vertebrae is most identical to the sheet-like branch of the SPRL in Hudiesaurus  (Upchurch et al. 2021). Notwithstanding the fact that Moore et al. (2018) noted several morphological differences between Bellusaurus and Klamelisaurus which are clearly non-ontogenetic despite the former being based on juvenile specimens, comparison by Moore et al. (2020) of Klamelisaurus with Mamenchisaurus sinocanadorum and Tienshanosaurus provides new insights into non-neosauropod eusauropod diversity in the Shishugou Formation in a few respect. For instance, the anterior caudal vertebrae of Klamelisaurus differ from those of Tienshanosaurus in lacking strong procoely in the anterior caudal vertebrae, given that strong procoely in the anterior and middle caudal vertebrae once used derived titanosaurs is also seen in many mamenchisaurids. Moreover, although the Klamelisaurus gobiensis and Mamenchisaurus sinocanadorum holotypes preserve non-overlapping cervical vertebrae, with four anterior cervicals included in the only known specimen of M. sinocanadorum, the two taxa come from different levels of the Shishugou Formation, indicating that there was some turnover in this geologic unit as far as the non-neosauropod eusauropod record is concerned, with Mamenchisaurus-like taxa from the upper part of the formation.

Bayesian inference-based cladistic analysis of Klamelisaurus by Moore et al. (2020) based on the Carballido et al (2015) matrix. Note that Euhelopus is recovered in the same clade as Klamelisaurus and Mamenchisaurus constructus (type species of Mamenchisaurus), whereas Bellusaurus falls within Macronaria

The results of the phylogenetic analyses conducted for Klamelisaurus gobiensis deserve attention because of the varying cladistic positions of some euhelopodids as well as Bellusaurus (whose precise cladistic position is stymied by the juvenile nature of all Bellusaurus specimens) in those phylogenies (which utilize the data matrices from the cladistic analyses by Carballido et al. 2015 and Gonzalez-Riga et al. 2018). In the implied-weights parsimony analysis based on the Gonzalez-Riga et al. data matrix, Euhelopodidae sensu D'Emic (2012) is recovered as an early-branching clade of Somphospondyli, but the implied-weights parsimony analysis based on the Carballido et al. data matrix as well as the equal-weights parsimony and Bayesian inference analyses recover Euhelopus and a few taxa of euhelopodids within Mamenchisauridae. On the other hand, Bellusaurus is recovered as a macronarian in all the topologies obtained by Moore et al. utilizing the Carballido et al. data matrix, but it is placed as a sister taxon of Diplodocoidea in the equal-weights and implied-weights parsimony analyses utilizing the Gonzalez et al. data matrix and as a sister taxon of Neosauropoda in the Bayesian inference analysis of the Gonzalez et al. data matrix. Although Moore et al. (2018) reserve judgment regarding the exact phylogenetic position of Bellusaurus due to the juvenile nature of specimens of this taxon, the recovery of Bellusaurus as a basal diplodocoid in some analyses is quite novel because until the description of the dicraeosaurid Lingwulong by Xu et al. (2018), no Jurassic diplodocoids were reported from East Asia. Even though Moore et al. acknowledge that Bellusaurus shares a handful of characters with some mamenchisaurids despite being distinct from Klamelisaurus and lacking features expected for juvenile Klamelisaurus, they note several characters that place Bellusaurus among neosauropods: (1) proatlantal facets on the otoccipital; (2) the lack of foramina between the basal tubera and basipterygoid processes; (3) posterior dorsal neural arches with steeply orientated postzygapophyses; (4) vertical struts within the lateral pneumatic foramen of the dorsal centra; (5) lateral branch of the centropostzygapophyseal lamina in middle and posterior dorsal neural arches; (6) a well-developed ambiens process of the pubis; and (7) fibular facet of the astragalus facing posterolaterally. If the recovery of Bellusaurus as a basal diplodocoid in some analyses by Moore et al. holds water in some future cladistic studies, the cranial architecture of Bellusaurus could shed light on how diplodocoids gradually evolved the elongated skull with slender, pencil-like teeth, given that Moore et al. find Turiasauria to fall within Diplodocoidea in both the equal-weights parsimony analysis of the Gonzalez-Riga data matrix and the implied-weights parsimony analysis of the Carballido et al. data matrix. The recovery of a few euhelopodids as sister to derived mamenchisaurids in some analyses by Moore et al., on the other hand, runs counter to previous cladistic studies placing Euhelopodidae sensu D'Emic (2012) at the base of Somphospondyli. Thus, the question arises: why the varying phylogenetic placements of some euhelopodids among the various topologies obtained by Moore et al. (2020)? 

D'Emic (2012) listed bifurcated neural spines and thick, subhorizontal epipophyseal–prezygapophyseal laminae on the cervical vertebrae as unambiguous synapomorphies uniting Euhelopus with Daxiatitan, Erketu, Phuwiangosaurus, Qiaowanlong, and Tangvayosaurus in a monophyletic Euhelopodidae to the exclusion of all other macronarians. The bifurcation of the cervical neural spines occurs in some mamenchisaurids and turiasaurians, but also various neosauropods, while the second character is present only in Erketu,  Qiaowanlong, and Phuwiangosaurus but not Euhelopus, which shares with Klamelisaurus thin epipophyseal–prezygapophyseal lamina passing nearly horizontally across the cervical neural arches. The extended implied-weights parsimony analysis by Moore et al. using the Gonzalez-Riga et al. matrix, despite agreeing with Wilson & Upchurch (2009) and D'Emic (2012) in recovering Euhelopus  inside Somphospondyli, does not recover Daxiatitan within Euhelopodidae sensu D'Emic (2012), and two of the three synapomorphies listed by D'Emic (2012) uniting Phuwiangosaurus as sister to Tangvayosaurus within Euhelopodidae are ambiguous because no caudal material is known for Erketu, Euhelopus, or Qiaowanlong, so it is unclear if those genera possess the synapomorphic caudal characters of Phuwiangosaurus or  Tangvayosaurus. Although Moore et al. note that Euhelopus and Klamelisaurus share a distolingual boss of the dentition, a rugose muscle scar extending anteriorly from the epipophysis to the posterior margin of the spinodiapophyseal fossa and ventrally convex prediapophyseal lamina of the middle and posterior cervical vertebrae, a ventrally bifurcated postzygodiapophyseal lamina of the cervicodorsal vertebrae, and a fourth femoral trochanter positioned near midline of posterior surface, they caution that the topology recovering Euhelopus as part of the "Core Mamenchisaurus-like Taxa" clade is weakly supported due to shared characters between Euhelopus and Klamelisaurus being present in a few members of Mamenchisauridae, raising the possibility of alternative affinities for Euhelopus. Poropat et al. (2022) note that the teeth of Euhelopus  are unusual for somphospondylan taxa in being spatulate-shaped, while a single tooth preserved in a specimen of Phuwiangosaurus siridhornae  described by Suteethorn et al. (2009) differs from non-somphospondylan macronarians in being peg-shaped. Therefore, it is probable that if Euhelopus is non-somphospondylan according to some phylogenetic analyses by Moore et al. (2020), it could be a basal macronarian outside as suggested by the cladistic analysis of Carballido et al. (2015) because Upchurch et al. (2021) note that the basal somphospondylan Yongjinglong also has a distolingual boss of the dentition, and the absence of caudal vertebrae preserved in the Euhelopus zdanskyi holotype raises the question of whether Euhelopus had strong procoely in the anterior and middle caudal vertebrae as in Klamelisaurus. 

References:

Carballido, J. L., Pol, D., Ruge, M. L. P., Bernal, S. P., Paramo-Fonseca, M. E., and  Etayo-Serna, F. 2015. A new Early Cretaceous brachiosaurid (Dinosauria, Neosauropoda) from northwestern Gondwana (Villa de Leiva, Colombia). Journal of Vertebrate Paleontology 35: e980505. doi:10.1080/02724634.2015.980505 

D’Emic, M. D. 2012. The early evolution of titanosauriform sauropod dinosaurs. Zoological Journal of the Linnean Society 166: 624–671. doi:10.1111/j.1096-3642.2012.00853.x

Dong, Z., Zhou, S., and Zhang, Y. 1983. Dinosaurs from the Jurassic of Sichuan. Palaeontologica Sinica, Series C 162: 1–136.

Gonzalez-Riga, B. J., Mannion, P. D., Poropat, S. F., David, O., D, L., and Coria, J. P., 2018. Osteology of the Late Cretaceous Argentinean sauropod dinosaur Mendozasaurus neguyelap: implications for basal titanosaur relationships. Zoological Journal of the Linnean Society 184 (1): 136–181. doi:10.1093/zoolinne/zlx103 

Moore, A. J., Mo, J., Clark, J. M. and Xu, X. 2018. Cranial anatomy of Bellusaurus sui (Dinosauria: Eusauropoda) from the Middle–Late Jurassic Shishugou Formation of northwest China and a review of sauropod cranialontogeny. PeerJ 6: e4881. doi:10.7717/peerj.4881 

Moore, A. J., P. Upchurch, P. M. Barrett, J. M. Clark, and Xu, X., 2020. Osteology of Klamelisaurus gobiensis (Dinosauria: Eusauropoda) and the evolutionary history of Middle–Late Jurassic Chinese sauropods. Journal of Systematic Palaeontology 18 (16):1299–1393.

Poropat, S.F., Frauenfelder, T.G., Mannion, P.D., Rigby, S.L., Pentland, A.H., Sloan, T. and Elliott, D.A., 2022. Sauropod dinosaur teeth from the lower Upper Cretaceous Winton Formation of Queensland, Australia and the global record of early titanosauriforms. Royal Society Open Science 9: 220381.

Suteethorn, S., Le Loeuff, J., Buffetaut, E., Suteethorn, V., Talumbook, C., and Chonglakmani, C., 2009. A new skeleton of Phuwiangosaurus sirindhornae (Dinosauria, Sauropoda) from NE Thailand. pp. 189-215. In: Buffetaut, E., Cuny, G., Le Loeuff, J., and Suteethorn, V. (eds), Late Palaeozoic and Mesozoic Ecosystems in SE Asia. Special Publication 315. London, UK: The Geological Society.

Upchurch, P., Barrett, P. M., and Dodson, P. 2004. Sauropoda. pp. 259–322. In: Weishampel, D.B., Dodson, P., and Osmolska, H. (eds), The Dinosauria, 2nd edition. University of California Press: Berkeley.

Upchurch P., Mannion, P.D., Xu, X., and Barrett, P.M., 2021. Re-assessment of the Late Jurassic eusauropod dinosaur Hudiesaurus sinojapanorum Dong, 1997, from the Turpan Basin, China, and the evolution of hyper-robust antebrachia in sauropods. Journal of Vertebrate Paleontology 41 (4): e1994414. doi:10.1080/02724634.2021.1994414

Wilson, J. A. & Upchurch, P., 2009. Redescription and reassessment of the phylogenetic affinities of Euhelopus zdanskyi (Dinosauria: Sauropoda) from the Early Cretaceous of China. Journal of Systematic Palaeontology 7(2): 199–239. doi:10.1017/S1477201908002691

Xu, X., Upchurch, P., Mannion, P. D., Barrett, P. M., Regalado-Fernandez, O. R., Mo, J., Ma, J., and Liu, H., 2018. A new Middle Jurassic diplodocoid suggests an earlier dispersal and diversification of sauropod dinosaurs. Nature Communications 9: 2700. doi:10.1038/s41467- 018-05128-1

Zhao, X., 1993. A new Middle Jurassic sauropod subfamily (Klamelisaurinae subfam. nov.) from Xinjiang Autonomous Region, China. Vertebrata PalAsiatica 31: 132–138.

Wednesday, June 29, 2022

The "flightless pterodactyl" that never was: Ornithopsis hulkei

Prior to and during the Victoria era, British fossil hunters came upon huge or peculiar bones of reptiles from Middle Jurassic to Early Cretaceous deposits in England that they interpreted as belonging to huge crocodile-like archosaurs, namely those from the Oolite Group of the Midlands, the Kimmeridge Clay of southern and eastern England, and the Wealden Supergroup of Sussex and the Isle of Wight. For instance, the type specimens of the basal eusauropod Cetiosaurus and the basal titanosauriform  Pelorosaurus were initially thought to have represented gigantic sea-going crocodiles, until more complete finds in the 1870s showed that they were actually dinosaurs and not crocodiles. However, most paleontology gurus overlook the fact that one Early Cretaceous titanosauriform sauropod from the UK, Ornithopsis, was misinterpreted by its describer as belonging not to a huge crocodile-like reptile, but instead as a flightless pterosaur!

Anterior view of the lectotype of Ornithopsis hulkei (NHMUK R28632) (from Owen 1875)

The story of the discovery and naming of Ornithopsis begins in the early 1850s, when an anterior dorsal vertebra was found in the Early Cretaceous (Barremian) Wessex Formation of the Isle of Wight along the English Channel coast of southern England and kept by Gideon Mantell (describer of Pelorosaurus) in his personal fossil collection, before being acquired by the British Museum in 1853 (a year after Mantell's death) and assigned the catalogue number BMNH R28632 (now NHMUK R28632). The dorsal vertebra, however, was not published in the scientific literature until Seeley (1870) erected the name Ornithopsis hulkei for NHMUK R28632 as well as NHMUK R2239, a dorsal vertebra found in the Early Cretaceous (late Valanginian) Tunbridge Wells Sand Formation of West Sussex in the 1820s by Gideon Mantell and misidentified by Owen (1854) as a quadrate of Iguanodon. He noted that NHMUK R28632 and NHMUK R2239 had cavities for air sacs seen in the bones of birds and pterosaurs, and thus surmised that Ornithopsis could be a missing link between pterosaurs and birds, but also possibly allied with dinosaurs, hence the name Ornithopsis meaning "bird face" in Greek.

Sir Richard Owen (1804-1892), who correctly determined that Ornithopsis was a sauropod dinosaur and not a flightless pterosaur

The identification of Ornithopsis as potentially being a flightless pterosaur would not hold water for very long, however. Owen (1875) agreed with Seeley (1870) that NHMUK R2239 was a dorsal vertebra rather than a quadrate, but he rejected Seeley's interpretation of Ornithopsis as a close relative of birds and pterosaurs and instead considered NHMUK R2239 and R28632 to be congeneric with his new sauropod genus Bothriospondylus from the Late Jurassic (Kimmerdgian) Kimmeridge Clay Formation of Wiltshire. The hypodigm for Ornithopsis hulkei was split into two species, with NHMUK R28632 receiving the new name Bothriospondylus magnus and NHMUK R2239 being made the holotype of the new species Bothriospondylus elongatus. For one thing, Richard Owen was a creationist and not a fan of Darwinist thought, so his lack of enthusiasm for Charles Darwin's theory of evolution endeared him to recognize that Ornithopsis belonged to a sauropod and not a pterosaur-like archosaur. Owen also must have been aware that because the Bothriospondylus elongatus holotype is from an older horizon than NHMUK R28632, the two vertebrae were most likely not conspecific. As a matter of fact, a year after he assigned the Ornithopsis hulkei material to Bothriospondylus, Owen (1876) changed his mind about B. magnus being congeneric with the Bothriospondylus type species (B. suffosus) and referred it to the sauropod genus Chondrosteosaurus from the same geologic horizon and location as NHMUK R28632. Forthwith, Ornithopsis would now be recognized not as a flightless pterodactyl, but instead as a member of Dinosauria --- although Richard Owen had been familiar with extinct and extant flightless birds, no one ever found a genuine pterosaur fossil with flightless abilities. 

In the 1860s and 1870s additional sauropod material was uncovered from the Wessex Formation of the Isle of Wight by Reverend William Fox and John Whitaker Hulke, including some vertebrae that would become the type specimens of the titanosauriforms Chondrosteosaurus magnus and Eucamerotus foxi. In his description of the new titanosauriform remains from the Isle of Wight, Hulke (1879) disputed Owen's opinion about the generic name Ornithopsis being misleading by pointing out that the syntypes of O. hulkei were lightly constructed regardless of the reclassification of Ornithopsis as a sauropod. He designated NHMUK R28632 as the lectotype of O. hulkei, making Bothriospondylus magnus a junior objective synonym of Ornithopsis, and the genera Chondrosteosaurus and Eucamerotus (the latter also described from the Isle of Wight) were synonymized with Ornithopsis. Although Hulke (1882, p. 375) treated the holotype of Bothriospondylus elongatus as the O. hulkei lectotype and referred NHMUK R28632 and the type material of Eucamerotus foxi the Wessex Formation of the Isle of Wight to his new species Ornithopsis eucamerotus, the earlier lectotype designation for O. hulkei by Hulke (1879) stands, as pointed out by Lydekker (1888). 

Although Ornithopsis had been wrongly interpreted as a flightless pterosaur when first named in 1870, it was nonetheless one of the first sauropod taxa to be described from the Isle of Wight and the fourth sauropod taxon described from the Early Cretaceous of Europe (after Pelorosaurus, Haestasaurus, and Oplosaurus). On a few occasions, Ornithopsis was synonymized with Pelorosaurus by von Huene (1909), Romer (1956), and Steel (1970) but Blows (1995) noted that the O. hulkei lectotype does not overlap with the holotype of Pelorosaurus conybeari and found Ornihopsis to be a distinct and valid genus of basal titanosauriform (followed by Upchurch et al. 2011).

References:

Blows, W.T., 1995. The Early Cretaceous brachiosaurid dinosaurs Ornithopsis and Eucamerotus from the Isle of Wight, England. Palaeontology 38 (1): 187–197.

Huene, F. v., 1909. Skizze zu einer Systematik und Stammesgeschichte der Dinosaurier. Centralblatt für Mineralogie, Geologie und Paläontologie 1909:12-22.

Hulke, J.W., 1879. Note (3rd) on (Eucamerotus, Hulke) Ornithopsis, H. G. Seeley, = Bothrospondylus magnus, Owen, = Chondrosteous magnus, Owen. Quarterly Journal of the Geological Society 35 (1–4): 752–762.

Hulke, J.W., 1882. Note on the Os Pubis and Ischium of Ornithopsis eucamerotus. Quarterly Journal of the Geological Society 38 (1–4): 372–376.

Lydekker, R. (1888). Catalogue of the Fossil Reptilia and Amphibia in the British Museum (Natural History). Part I. Containing the Orders Ornithosauria, Crocodilia, Dinosauria, Squamata, Rhynchocephalia, and Proterosauria. British Museum (Natural History). Department of Geology. 309 pp.

Owen, R., 1854. Monograph on the Fossil Reptilia of the Wealden Formations. Part II. Dinosauria (Iguanodon).  Monographs of the Palaeontographical Society 8 (27): 1–54.

Owen, R., 1875. Monographs on the British Fossil Reptilia of the Mesozoic Formations. Part II. (Genera Bothriospondylus, Cetiosaurus, Omosaurus). Monographs of the Palaeontographical Society 29 (133): 15–93.

Owen, R., 1876. Monograph on the Fossil Reptilia of the Wealden and Purbeck Formations. Supplement No. VII. Crocodilia (Poikilopleuron) and Dinosauria? (Chondrosteosaurus). Monographs of the Palaeontographical Society 30 (136): 1–7.

Romer, A.S., 1956. Osteology of the Reptiles. University of Chicago Press: Chicago: IL 772 pp. 

Seeley, H.G., 1870. Ornithopsis, a gigantic animal of the Pterodacyle kind from the Wealden. Annals and Magazine of Natural History 5 (4): 305–318.

Steel, R., 1970. Part 14. Saurischia. Handbuch der Paläoherpetologie. Gustav Fischer Verlag: Stuttgart, 87 pp.

Upchurch, P., Mannion, P.D., and Barrett, P.M., 2011. Sauropod dinosaurs. pp. 476–525. In: Batten, D.J. (ed.). English Wealden Fossils. The Palaeontological Association.

Tuesday, June 28, 2022

Personal thoughts on Amphicoelias paper by Mannion et al. (2021)

During the Bone Wars in the late 1800s, Edward Drinker Cope (1840-1897) and Othniel Charles Marsh (1831-1899) described several sauropod taxa from the Morrison Formation of western North America, with Marsh erecting the most sauropod species from the Morrison. Although several sauropod genera erected by Marsh have stood the taxonomic test of time, like Apatosaurus, Barosaurus, Brontosaurus, and Diplodocus, the only sauropod genus from the Morrison Formation named by Cope whose validity has been upheld is Camarasaurus, while Caulodon has been synonymized with Camarasaurus (but see here). One sauropod genus described from the Morrison Formation by E.D. Cope whose taxonomic status has fluctuated over time, however, is Amphicoelias Cope, 1877. Although Amphicoelias is poorly known in terms of the holotype of its type species, A. altus, being representing by a few elements, one nominal species of Amphicoelias, A. fragillimus, enjoyed conjectural fame as a super-giant diplodocid until Carpenter (2018) drastically reduced the size estimates for this taxon to 102 feet (31 meters) and reclassified it as a rebbachisaurid, erecting the new genus Maraapunisaurus for it. On the other hand, the validity and precise systematic position of Amphicoelias has been debated, with some studies placing it as a basal diplodocoid and others recovering it as diplodocid. Recently, a new paper on the anatomy and systematics of Amphicoelias was published by Mannion et al. (2021), and while it reaffirms the validity of Amphicoelias as upheld by several authors, I have taken the liberty of expressing some thoughts about the Mannion et al. paper regarding Amphicoelias with respect to diagnostic characters, phylogenetic position, and the bearing of studies on Morrison diplodocoid ontogeny upon Morrison sauropod diversity. 

Selected elements of the holotype of Amphicoelias altus (AMNH 5764): posterior dorsal vertebra (top) and right femur (bottom) (from Mannion et al. 2021)

In the section of their paper in which they redescribe the holotype of Amphicoelias altus (AMNH 5764), Mannion et al. list the "femoral shaft with subcircular cross-section" as one of three autapomorphies for Amphicoelias in the revised diagnosis for this taxon, noting that the femur of AMNH 5764 differs from described Morrison diplodocoid taxa in having a ratio of the mediolateral to anteroposterior diameter of the femur being 0.99 to 1.1 (despite a few signs of taphonomic crushing). However, they also note that the dicraeosaurid specimen MOR 592 found in Montana also has a femur whose cross-section is subcircular at the midshaft; in fact, the subcircular cross-section of the femur was used by Wilson and Smith (1996) to justify referring MOR 592 to Amphicoelias and conclude that Amphicoelias was a basal diplodocoid based on cladistic results that were never published. However, Whitlock (2011) assigned MOR 592 to the family Dicraeosauridae due to the presence of a sharp supraoccipital crest and a symphyseal tuberosity on the dentary, although Woodruff & Fowler (2012) and Woodruff et al. (2017) regarded MOR 592 as an immature diplodocine specimen, but nevertheless recovered Amphicoelias as a basal diplodocoid more derived than Haplocanthosaurus and Amazonsaurus. According to Mannion et al. (2021), the ratio of the mediolateral to anteroposterior diameter of the femur of MOR 592 is approximately 1.3, slightly greater than that for Amphicoelias altus, and MOR 592 has a femur with a slightly beveled distal end in contrast to the more pronounced beveling of the distal femur of AMNH 5764. On the other hand, Tschopp et al. (2015) note that the holotype of Brontosaurus parvus (CM 566) also has a subcircular femoral cross-section, while Wilhite (2005) reports that the subcircular femoral cross-section observed in Amphicoelias, the Brontosaurus parvus holotype, and MOR 592 also occurs in a few diplodocid femora from the Dry Mesa Quarry in Colorado. Since Amphicoelias is recovered as either a basal diplodocid by Tschopp et al. (2015) or an apatosaurine diplodocid by Tschopp and Mateus (2017), whereas Amphicoelias is variously recovered as a stem diplodocoid more derived than Haplocanthosaurus or a diplodocid by Mannion et al. (2021), the subcircular femoral cross-section described for Amphicoelias most likely evolved convergently among a few taxa within Flagellicaudata because Amphicoelias altus is distinguished by Mannion et al. (2021) from all other diplodocoids in having the apex of the posterior dorsal neural spine with rounded, non-tapered lateral projections resulting from the expansion of spinodiapophyseal laminae and little material is preserved in AMNH 5764.

Stratigraphic chart of dinosaur localities in the Morrison Formation (from Turner and Peterson 1999). Despite the opinion of some that the diversity of diplodocoids in the Morrison Formation has been inflated, the type localities of Haplocanthosaurus delfsi (CO-5) and Brontosaurus yahnanpin (WY-44) are stratigraphically low in the Morrison Formation, and type locality of Amphicoelias altus (CO-71) is situated near the top of the Brushy Basin Member of the Morrison Formation, being stratigraphically higher than the type localities of Apatosaurus ajax, A. louisae, Brontosaurus excelsus, and B. parvus. Moreover, three different groups of the diplodocoids (haplocanthosaurids, diplodocids, and dicraeosaurids) have been found at the Felch Quarry 1 (CO-3) in Garden Park, Colorado.  

When addressing the question of whether or not some Morrison diplodocoid species are growth stages of well-known taxa as hinted by Woodruff (2019), Mannion et al. stress that the basal position of the genus Haplocanthosaurus within Diplodocoidea is not attributable to ontogeny given that known specimens of H. priscus and H. delfsi are of the adult/near-adult stage. When taking into account the cladistic diversity and stratigraphic distribution of sauropods within the Morrison Formation, it should be noted that Brontosaurus (=Eobrontosaurus) yahnahpin and Haplocanthosaurus delfsi hail from the lower half of the upper part of the Salt Wash Member of the Morrison Formation whereas Amphicoelias altus was found near the top of the Brushy Basin Member (Turner and Peterson 1999, fig. 7) and that no members of Turiasauria or Mamenchisauridae have yet been reported from the Morrison Formation, although the Lourinhã and Tendaguru Formations have yielded members of Diplodocoidea, Macronaria and Turiasauria. Additionally, given that Whitlock and Wilson Mantilla (2020) note that the juvenile diplodocine specimens CM 3452 and CM 11255 (the latter probably Barosaurus; Melstrom et al. 2016) differ from Kaatedocus, Smitanosaurus, Suuwassea, and MOR 592 in lacking a postparietal foramen despite being juveniles, although the adult apatosaurine specimen BYU 17096 has this feature, it is not hard to imagine four dicraeosaurid taxa existing in the Morrison Formation because known specimens of Kaatedocus, Smitanosaurus, and MOR 592 were found in the upper part of the Salt Wash Member and lowermost part of the Brushy Basin Member, whereas Suuwassea probably was found high in the Morrison Formation (Harris and Dodson 2004; Turner and Peterson 1999). While I agree with Mannion et al. (2021) that ontogeny is an important factor to take into account when determining whether small or primitive sauropod specimens from the Morrison Formation are juveniles of existing species or more basal than well-known diplodocids, the assignment of Suuwassea and MOR 592 to Dicraeosauridae by Whitlock (2011) took into account the possibility that the sub-adult status of the Suuwassea holotype was why Suuwassea defied precise classification within Diplodocoidea when first described by Harris and Dodson (2004), while bearing in mind the fact that some characteristics used to refer MOR 592 to Amphicoelias by Wilson and Smith (1996) were likely to be found in other diplodocoid taxa. Moreover, since Brontosaurus yahnanpin was found lower in the Morrison Formation than Amphicoelias or other species of Brontosaurus, it is possible that it is actually more basal than either B. excelsus, B. parvus, or Apatosaurus because the holotype of Amphicoelias altus contains a few skeletal elements and was found in the uppermost layer of the Brushy Basin Member.     

References:

Carpenter, K., 2018. Maraapunisaurus fragillimus, N.G. (formerly Amphicoelias fragillimus), a basal Rebbachisaurid from the Morrison Formation (Upper Jurassic) of Colorado. Geology of the Intermountain West 5: 227–244.

Harris, J.D. and Dodson, P., 2004. A new diplodocoid sauropod dinosaur from the Upper Jurassic Morrison Formation of Montana, USA. Acta Palaeontologica Polonica 49 (2): 197–210.

Mannion P.D., Tschopp E., and Whitlock, J.A. 2021. Anatomy and systematics of the diplodocoid  Amphicoelias altus supports high sauropod dinosaur diversity in the Upper Jurassic Morrison Formation of the USA. Royal Society Open Science 8 (6): Article ID 210377.  doi:10.1098/rsos.210377        

Melstrom, K.M., D’Emic, M.D., Chure, D.J., and Wilson, J.A., 2016. A juvenile sauropod dinosaur from the Late Jurassic of Utah, USA, presents further evidence of an avian style air-sac system. Journal of Vertebrate Paleontology e1111898.

Tschopp, E., Mateus, O., and Benson, R.B.J., 2015. A specimen-level phylogenetic analysis and taxonomic revision of Diplodocidae (Dinosauria, Sauropoda).  PeerJ  3:e857    

Tschopp, E., and Mateus, O., 2017. Osteology of Galeamopus pabsti sp. nov. (Sauropoda: Diplodocidae), with implications for neurocentral closure timing, and the cervico-dorsal transition in diplodocids. PeerJ 5:e3179 

Turner, C.E. and Peterson, F., 1999. Biostratigraphy of dinosaurs in the Upper Jurassic Morrison Formation of the Western Interior, U.S.A. pp. 77–114. In: Gillette, D.D. (ed.), Vertebrate Paleontology in Utah. Utah Geological Survey Miscellaneous Publication 99-1.

Wilhite, D.R. 2005. Variation in the appendicular skeleton of North American sauropod dinosaurs: taxonomic implications. pp. 268-301. In: Tidwell, V., and Carpenter, K. (eds.), Thunder-lizards: the Sauropodomorph dinosaurs. Indiana University Press, Bloomington.

Wilson, J.A., and Smith, M., 1996. New remains of Amphicoelias Cope (Dinosauria: Sauropoda) from the Upper Jurassic of Montana and diplodocoid phylogeny. Journal of Vertebrate Paleontology 16 (supp. to volume 3): 73A.

Whitlock, J. A. 2011. A phylogenetic analysis of Diplodocoidea (Saurischia: Sauropoda). Zoological Journal of the Linnean Society 161: 872–915.

Whitlock, C., and Wilson Mantilla, J., 2020. The Late Jurassic sauropod dinosaur  'Morosaurus’  agilis  Marsh, 1889 reexamined and reinterpreted as a dicraeosaurid. Journal of Vertebrate Paleontology 40  (6) DOI: 10.1080/02724634.2020.1780600

Woodruff, C., and Fowler, D. W. 2012., Ontogenetic influence on neural spine bifurcation in Diplodocoidea (Dinosauria: Sauropoda): A critical phylogenetic character. Journal of Morphology 273: 754–764. 
 
Woodruff, D. C., Fowler, D. W. and Horner, J. R., 2017. A new multi-faceted framework for deciphering diplodocid ontogeny. Palaeontologia Electronica 20.3.43A: 1–53.

Friday, February 11, 2022

Abditosaurus and implications for the paleobiogeography of Late Cretaceous lithostrotians from Europe

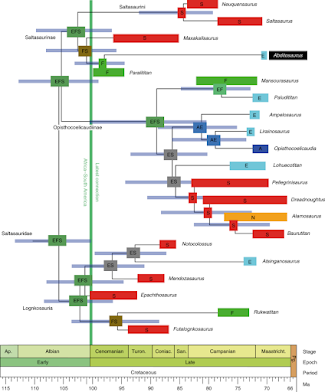
Since the 1990s a plethora of titanosaur taxa have been described from the Late Cretaceous (latest Campanian-Maastrichtian) of northeastern Spain and southern France (which constituted the Ibero-Armorican island during the latest Cretaceous) as well as Transylvania, Romania, adding to the hitherto described taxa Hypselosaurus from the Provence region of southern France and Magyarosaurus from Transylvania, Romania. Until recently, however, the interrelationships of lithostrotian taxa from the Late Cretaceous of Europe was not tested within a cladistic framework, with most published cladistic studies including only Ampelosaurus and Lirainosaurus (see cited references in Díez Díaz et al. 2018). The cladistic analysis of Sallam et al. (2018) resolved Ampelosaurus, Lirainosaurus, Lohuecotitan, and Paludititan as saltasaurids closely related to Mansourasaurus from the Late Cretaceous of Egypt, implying a geographic dispersal of some lithostrotians from southern Europe into North Africa during the Late Cretaceous. Meanwhile, a cladistic analysis by Díez Díaz et al. (2018) found Ampelosaurus,  Atsinganosaurus, and Lirainosaurus to form a distinct clade within Saltasauridae that they named Liranosaurinae, whereas the taxa Lohuecotitan and Paludititan were resolved as more derived than the basalmost lithostrotian Malawisaurus but cladistically more primitive than derived lithostrotians. This week, another new lithostrotian titanosaur from the latest Cretaceous of southern Europe came hot off the press, named Abditosaurus kuehnei (Vila et al. 2022), and instead of being a dwarf, insular taxon, it surprisingly happens to be a giant for its time and geographical location. Therefore, this post will discuss the implications of Abditosaurus for the paleobiogeography of lithostrotians from the latest Cretaceous of Europe.

Walter Georg Kühne (1911–1991), the discoverer of the holotype of Abditosaurus kuehnei

As noted by Vila et al. (2022; supplementary material), the history of the discovery of the holotype of  Abditosaurus kuehnei is rather lengthy and tortuous, hampered by funding issues and bad weather. In September 1954, German paleontologist Walter Georg Kühne, an expert on Mesozoic mammals from Europe and worldwide, prospected Cretaceous outcrops west of the village of Orcau in the Tremp Basin of Catalonia, Spain, with the goal of finding Cretaceous mammal fossils when he unexpectedly found fossils of a titanosaur sauropod. For the next two weeks (September 27 to October 5), he unearthed ten bones at the Orcau-1 site, of which two chevrons, a right tibia, and a distal left femur were collected and sent to the Instituto Lucas Mallada (ILM, now Museo Nacional de Ciencias Naturales [MNCN]) in Madrid, and other remains (e.g. proximal left femur, left humerus, two articulated dorsal vertebrate) were left at the site. Kühne returned to the Orcau-1 site and excavated a complete right femur and humerus, a distal left fibula, the anterior end of a left scapula, a chevron, an indeterminate “short” bone, a few small iliac fragments, a complete dorsal vertebra, and fragments of three dorsal ribs, which were also sent to the ILM. He requested additional excavations at the Orcau-1 site, but a lack of funds caused field work at the locality to be shelved. Lapparent and Aguirre (1956, 1957) considered the titanosaur material from the Orcau-1 site to be a probable new species of the genus Hypselosaurus Matheron, 1869 (now considered a nomen dubium; Le Loeuff 1993). In 1984 and 1986 Josep Vicenç Santafé of the Institut de Paleontologia de Sabadell in Barcelona and members of the Institut d’Estudis Ilerdencs in Lleida revisited the Orcau-1 locality; the 1986 expedition, which lasted for five days, unearthed part of a sternal plate and three dorsal ribs (of which one, MCD-6985, was collected and deposited in the Museu de la Conca Dellà). From 2012 to 2014, members from the Institut Català de Paleontologia, the Universidad de Zaragoza, and the Museu de la Conca Dellà conducted six consecutive expeditions to the Orcau-1 site, unearthing the remaining axial and appendicular remains from the locality and the remains left at the site by Kühne and Santafé, including an articulated cervicodorsal series, additional limb and pectoral girdle remains, tooth fragments, and ribs, all of which were sent to the MNCN. The chevrons (MNCN 59295, MNCN 59539, and MNCN 62760) and humerus (MNCN 79834) unearthed by Kühne were assigned to Titanosauriformes indet. and Titanosauria indet. respectively by Martín Jiménez et al. (2017). The cervicodorsal series of the holotype of Abditosaurus kuehnei constitutes the most complete neck for any titanosaur described from the latest Cretaceous of Europe given that complete or nearly complete necks have been described for very few sauropod specimens (Taylor 2022). 

Phylogenetic analysis of Abditosaurus kuehnei and other derived lithostrotian taxa (after Vila et al. 2022)

In their phylogenetic analysis of Titanosauria, Vila et al. recover Abditosaurus as the sister taxon of the Paralititan from the middle Cretaceous (Cenomanian) of Egypt within Saltasaurinae sensu Gorcsak & O'Connor (2019), while Ampelosaurus, Lirainosaurus, Lohuecotitan, and Paludititan are recovered within Opisthocoelicaudiinae and Atsinganosaurus is placed within Lognkosauria as the sister taxon of Notocolossus. Because Sallam et al. (2018) recover all lithostrotian taxa from the Late Cretaceous of Europe except Atsinganosaurus within the same clade as Mansourasaurus, the cladistic analysis by Vila et al. (2022) suggests that more than large/medium-size lithostrotian clade dispersed into Europe from Africa, as Paludititan and Mansourasaurus are recovered by Vila et al. (2022) in a basal position to a clade formed by Ampelosaurus, Lirainosaurus, Lohuecotitan, and the South American taxa Baurutitan, Dreadnoughtus, and Pellegrinisaurus within Opisthocoelicaudiinae sensu Gorcsak & O'Connor. The notion of some Gondwanan tetrapod groups dispersing into the Europe during the late Cretaceous is not new; the assignment of the crocodyliform Doratodon carcharidens to the predominantly Gondwanan clade Notosuchia shows that some notosuchians immigrated to Europe from North Africa (Rabi and Sebők 2015), while abelisauroids are represented in the Late Cretaceous of France by Arcovenator and Tarascosaurus (see Tortosa et al. 2014). Since Opisthocoelicauda is resolved as more closely related to some of the taxa included in Lirainosaurinae by Díez Díaz et al. (2018) than to either Paludititan or Mansourasaurus, and Wang et al. (2021) recover the East Asian taxa Abdarainurus and Huabeisaurus as sister to the basal titanosaur Andesaurus from the middle Cretaceous (Cenomanian) of Argentina, it's reasonable to assume that two lineages of large/medium-bodied lithostrotians dispersed into Europe from Gondwana during Late Cretaceous because Normanniasaurus from the middle Cretaceous (Albian) of northern France and Volgatitan from the Early Cretaceous (Hauterivian) of European Russia are recovered as sister to Colossosauria by Averianov & Efimov (2018) and Mannion et al. (2019), while Mocho et al. (2019) recover two indeterminate titanosaur specimens from the late Aptian-Cenomanian of Spain and Italy as more closely related to Rapetosaurus than to Colossosauria.    

When comparing the results of the cladistic analysis by Vila et al. (2022) to the phylogenetic results obtained by Díez Díaz et al. (2018), I should emphasize that the difference between the two studies in terms of the phylogenetic placement of Lohuecotitan and Paludititan relative to the taxa included in Lirainosaurinae by Díez Díaz et al. is best explained by the huge amount of missing data for the cranial and cervical vertebral characters for several Late Cretaceous titanosaur taxa from Europe in the data matrix employed for the Díez Díaz et al. (2018) analysis, the number of non-European lithostrotian taxa selected for the cladistic analysis, and the fact that the recovery of Nemegtosaurus as the sister taxon to Rapetosaurus in several phylogenies (e.g. Wilson 2002) is now known to be artificial because more than one clade of lithostrotians had a Rapetosaurus-like skull. Given that the Abditosaurus kuehnei holotype preserves the only complete or near-complete neck for any Late Cretaceous titanosaur from the western Tethyan archipelago, and unpublished cladistic results concur with Vila et al. (2022) in recovering Lohuecotitan and Paludititan as part of the same lithostrotian clade as Mansourasaurus and Opisthocoelicauda, it is possible that currently undescribed titanosaur specimens from the Lo Hueco locality could shed new light on the cervical morphology of taxa assigned to Lirainosaurinae. For one thing, Atsinganosaurus is recovered as sister to Ampelosaurus and Lirainosaurus by Díez Díaz et al. (2018) but falls as sister to Colossosauria in the Vila et al. (2022), and because Díez Díaz et al. (2018) note that material referred to Atsinganosaurus by Garcia et al. (2010) was not found articulated or associated with the A. velauciensis holotype (comprising four posterior dorsal vertebrae), it is possible that some of the specimens referred to this taxon might instead belong to Abditosaurus. 

In summary, more than one clade of large- and medium-sized lithostrotian titanosaurs immigrated to Europe from Gondwana during the Late Cretaceous, gradually supplanting dwarf, insular genera like Magyarosaurus by the latest Maastrichtian. Although insular dwarfism is prevalent among some lithostrotian taxa from the Late Cretaceous of Europe, the size estimates and phylogenetic position for Abditosaurus demonstrate that the environment of the Ibero-Armorican Island most likely did not pose an ecological obstacle to giant titanosaurs dispersing from Gondwana because titanosaur specimens from the middle Cretaceous of Italy and Spain and phylogenetic affinities of Normanniasaurus to colossosaurians indicate that multiple lithostrotian clades dispersed into Europe by the Albian. Future discoveries and re-evaluation of lithostrotian titanosaur specimens currently seen as indeterminate may further shed light the palebiogeographic patterns of lithostrotians from the Late Cretaceous of Europe.   

References:

Averianov, A., and V. Efimov, 2018. The oldest titanosaurian sauropod of the Northern Hemisphere.  Biological Communications 63(6):145–162. doi:10.21638/spbu03.2018.301.

Díez Díaz, V., Garcia, G., Pereda-Suberbiola, X., Jentgen-Ceschino, B., Stein, K., Godefroit, P., and Valentin, X., 2018. The titanosaurian dinosaur Atsinganosaurus velauciensis (Sauropoda) from the Upper Cretaceous of southern France: New material, phylogenetic affinities, and palaeobiogeographical implications. Cretaceous Research. 91: 429–456. doi:10.1016/j.cretres.2018.06.015

Garcia, G., Amico, S., Fournier, F., Thouand, E., and Valentin, X., 2010. A new titanosaur genus (Dinosauria, Sauropoda) from the Late Cretaceous of southern France and its paleobiogeographic implications. Bulletin de la Societe Geologique de France 181(3):269–277.

Gorscak, E., and O’Connor, P.M., 2019. A new African titanosaurian sauropod dinosaur from the middle Cretaceous Galula Formation (Mtuka Member), Rukwa Rift Basin, southwestern Tanzania.  PLoS ONE 2 (14): e0211412. doi:10.1371/journal.pone.0211412 

Lapparent, A. F. de, and Aguirre, E. S. J., 1956. Algunos yacimientos de Dinosaurios en el Cretacico Superior de la Cuenca de Tremp. (Prov. de Leirida, Espana). Estud. Geol. Inst. Invest. Lucas Mallada 12 (31-32): 37-382.

Lapparent, A. F. de, and Aguirre, E. S. J., 1957. Presence de Dinosauriens dans le Cretace superieur du bassin de Tremp (province de Lerida, Espagne). Compte rendu sommaire des seances de la Societe de Geologie, France 1956: 261-262.

Le Loeuff, J., 1993. European titanosaurids. Revue de Paléobiologie, Volume Spéciale 7:105-117.

Mannion, P. D., Upchurch, P., Jin, X., and Zheng, W., 2019. New information on the Cretaceous sauropods of Zhejiang Province, China: impact on Laurasian titanosauriform phylogeny and biogeography. Royal Society Open Science 6(8):191057. doi:10.1098/rsos.191057.

Martín Jiménez, M., Sánchez-Chillón, B., Escaso, F., Mocho, P., Narváez, I., Ortega, F., and Pérez-García, A., 2017. Systematic study of the historical material of Upper Cretaceous reptiles from the Tremp Basin (Catalonia, Spain) housed at the Museo Nacional de Ciencias Naturales (Madrid). Journal of Iberian Geology 43(2): 217-233. 

Mocho, P., A. Pérez-García, M. Martín Jiménez, and F. Ortega, 2019. New remains from the Spanish Cenomanian shed light on the Gondwanan origin of European Early Cretaceous titanosaurs. Cretaceous Research 95:164–190. doi:10.1016/j.cretres.2018.09.016.

Rabi, M., and Sebők, N., 2015. A revised Eurogondwana model: Late Cretaceous notosuchian crocodyliforms and other vertebrate taxa suggest the retention of episodic faunal links between Europe and Gondwana during most of the Cretaceous. Gondwana Research. 28 (3): 1197–1211.  doi:10.1016/j.gr.2014.09.015

Sallam, H., Gorscak, E., O'Connor, P., El-Dawoudi, I., El-Sayed, S., Saber, S., 2018. New Egyptian sauropod reveals Late Cretaceous dinosaur dispersal between Europe and Africa. Nature 2 (3): 445–451. doi:10.1038/s41559-017-0455-5

Taylor, M., 2022. Almost all known sauropod necks are incomplete and distorted. PeerJ 10:e12810  .

Tortosa, T., Buffetaut, E., Vialle, N., Dutour, Y., Turini, E., and Cheylan, G., 2014. A new abelisaurid dinosaur from the Late Cretaceous of southern France: Palaeobiogeographical implications. Annales de Paléontologie 100(1): 63-86.

Vila, B., Sellés, A., Moreno-Azanza, M., Razzolini, N.L., Gil-Delgado, A., Canudo, J.I., and Galobart, A., 2022. A titanosaurian sauropod with Gondwanan affinities in the latest Cretaceous of Europe. Nature Ecology & Evolution 6: 288-296. doi:10.1038/s41559-021-01651-5.

Wang, X., K. L. N. Bandeira, R. Qiu, S. Jiang, X. Cheng, Y. Ma, and A. W. A. Kellner. 2021. The first dinosaurs from the Early Cretaceous Hami Pterosaur Fauna, China. Scientific Reports 11:14962. doi:10.1038/s41598-021-94273-7.

Wilson, J.A., 2002. Sauropod dinosaur phylogeny: critique and cladistic analysis. Zoological Journal of the Linnean Society 136 (2): 215–275.

Saturday, December 18, 2021

Critical analysis of the Navarro (2019) thesis regarding Tapuiasaurus

A titanosaur specimen (MZSP-PV 807) from the Early Cretaceous (late Barremian-early Aptian) Quiricó Formation in Minas Gerais, southeastern Brazil was described as the holotype of the new genus and species Tapuiasaurus macedoi by Zaher et al. (2011). In the original description (focused solely on the skull), Zaher et al. recovered this taxon as a member of Nemegtosauridae sensu Wilson (2002), but the cladistic placement of Tapuiasaurus as sister to Nemegtosaurus rather than Rapetosaurus created a 55 million year ghost lineage, and Poropat et al. (2015) recovered Rapetosaurus as a sister taxon of Isisaurus within Saltasauridae and Nemegtosaurus as more basal among advanced lithostrotians, indicating that cranial characters cited as diagnostic for Nemegtosauridae by Wilson (2002) occur in more than one lithostrotian clade. Wilson et al. (2016) provided a more detailed description of the skull of the Tapuiasaurus macedoi, and utilizing new morphological data, they re-analyzed the cladistic position of Tapuiasaurus and found it to be extremely labile, further confirming that Tapuiasaurus was not as closely related to Nemegtosaurus as previously thought. Meanwhile in their description of the lithostrotian Sarmientosaurus from Argentina, Martinez et al. (2016) also recovered Tapuiasaurus as distantly related to Nemegtosaurus. In an unpublished thesis describing of the postcranial skeleton of Tapuiasaurus, Navarro (2019) agrees with Wilson et al. (2016) that Tapuiasaurus is distantly related to Nemegtosaurus, but finds Tapuiasaurus to fall in a more basal position within Lithostrotia along with Isisaurus and Rapetosaurus. Given that the inter-relationships among derived titanosaurs are still a work in progress despite recent advances, I will allow the main findings of the phylogenetic analysis of Tapuiasaurus by Navarro (2019) and their implications for lithostrotian macroevolution do the talking, especially in light of the recent paper by Poropat et al. (2021) recovering Sarmientosaurus outside Lithostrotia as the sister taxon of Diamantinasaurus.

Skull of the holotype of Tapuiasaurus macedoi (MZSP-PV 807) (after Zaher et al. 2011)

In the cladistic analysis in part 4 of his thesis (titled "Results"), Navarro (2019) recovers Tapuiasaurus as the sister taxon of the East Asian taxon Yongjinglong and an unnamed lithostrotian titanosaur from the Adamantina Formation of the Prata municipality in southeastern Brazil, with all three taxa forming a clade sister to Isisaurus and Rapetosaurus. He erects the nomen ex dissertationae "Tapuiasaurinae" to include Tapuiasaurus, Yongjinglong, the Prata titanosaur, and probably Gobititan, and the clade formed by "Tapuiasaurinae", Isisaurus, and Rapetosaurus falls as phylogenetically intermediate between the most basal lithostrotians (Malawisaurus and Rukwatitan) from East Africa and the most derived lithostrotians (Eutitanosauria sensu Navarro 2019). The recovery of Isisaurus and Rapetosaurus as outside Saltasauridae (contra Poropat et al. 2015) adds a new twist in understanding lithostrotian macroevolution, because their placement as sister to "Tapuiasaurinae" would imply that more than one clade of lithostrotian titanosaurs acquired Nemegtosaurus/Rapetosaurus-like cranial features by the Aptian-Albian interval, since Yongjinglong hails from the Aptian-Albian upper part of the Hekou Group of northern China, and hence temporally intermediate between Tapuiasaurus and Rapetosaurus.  Yongjinglong itself was originally described as an opisthocoelicaudiine saltasaurid by Li et al. (2014) but was recovered outside Titanosauria as a euhelopodid by Mannion et al. (2019). Although the vast majority of colossosaurian titanosaurs are based on specimens that include no skull material, a recent paper by Averianov et al. (2021) recovering the Early Cretaceous (Hauterivian) genus Tengrisaurus as a relative of Colossosauria suggests that both saltasaurids and non-saltasaurids diverged from the most basal lithostrotians and the Isisaurus+Rapetosaurus+"Tapuiasaurinae" clade by the Hauterivian, in which case complete skull material for many colossosaurian taxa is required to determine how the cranial anatomy of colossosaurians compares to that of saltasaurids, Rapetosaurus and Tapuiasaurus. 

With respect to the systematic paleontology section of Chapter 1 in Navarro's (2019) thesis, the genera Adamantisaurus, Arrudatitan, and Trigonosaurus are grouped together in a distinct clade that is sister to Rinconsauria, dubbed "Trigonosaurinae". However, Aeolosaurus and Gondwanatitan are not included by Navarro in his cladistic analysis even though he offers a stem-based definition for Aeolosaurini (under which only Aeolosaurus and Gondwanatitan are included), and cladistic analyses by França et al. (2016), Hechenleitner et al. (2020), Silva et al. (2021), and Soto et al. (2022)  recover these genera as closely related to the taxa included by Navarro (2019) in Rinconsauria and "Trigonosaurinae", with the latter two papers grouping Trigonosaurus with Bravasaurus, Gondwanatitan, and Uberabatitan  rather than Aeolosaurus and Arrudatitan. Since the thesis by Navarro (2019) is unpublished, and the holotype of Aeolosaurus rionegrinus is less complete than that of Gondwanatitan faustoi, the proposed clade "Trigonosaurinae" is best treated with a high level of caution, considering that the material preserved in the holotype of Adamantisaurus (MUGEO 1282) is far less substantial than that of Arrudatitan and Trigonosaurus.

In his discussion of the comparisons of the postcranial skeleton of Tapuiasaurus with other titanosaurs, Navarro notes that the manus of the Tapuiasaurus macedoi holotype differs from that described for the Australian titanosaur Diamantinasaurus in having manual phalanges in the first metacarpal (unlike the 2-2-2-2-2 phalangeal formula described for Diamantinasaurus), while noting that Opisthocoelicauda has a manus with reduced ossified phalanges (see Poropat et al. 2015). Although he notes that the vast majority of titanosaur taxa do not preserve manual material, he interprets the phalangeal formula of Tapuiasaurus as reflective of a gradual reduction of the manus as a derived condition for titanosaurs more derived than Andesaurus and Diamantinasaurus. The holotype of Savannasaurus elliotorum, which hails from the same geologic unit and location as Diamantinasaurus, also has the phalangeal formula of Diamantinasaurus (Poropat et al. 2016). Although Diamantinasaurus and Savannasaurus are recovered in a distinct titanosaur clade (Diamatinasauria) outside Lithostrotia as more derived than Andesaurus rather than sister taxa of Andesaurus as in Navarro (2019), and no phalangeal remains are known for Andesaurus or Ninjatitan, the phylogenetic placement of Tapuiasaurus by Navarro (2019) is apparently consistent with Navarro's conclusion that the most primitive titanosaurs retained a 2-2-2-2-2 phalangeal formula. Likewise, Navarro (2019) notes that the pes of Tapuiasaurus differs from derived lithostrotians like Alamosaurus, Mendozasaurus, and Opisthocoelicauda in having 10 phalanges (as does Gobititan), concluding that Tapuiasaurus exhibits a combination of a gradually reduced manus and a pes with 10 phalanges (reduced in more derived lithostrotians).

References:

Averianov, A. O., Sizov, A. V., and Skutschas, P. P., 2021. Gondwanan affinities of Tengrisaurus, Early Cretaceous titanosaur from Transbaikalia, Russia (Dinosauria, Sauropoda). Cretaceous Research 122:104731. doi:10.1016/j.cretres.2020.104731

França, M.A.G., Marsola, J.C.d.A., Riff, D., Hsiou, A.S., and Langer, M.C., 2016. New lower jaw and teeth referred to Maxakalisaurus topai (Titanosauria: Aeolosaurini) and their implications for the phylogeny of titanosaurid sauropods. PeerJ 4:e2054. doi:10.7717/peerj.2054

Hechenleitner, E.M., Leuzinger, L., Martinelli, A.G., Rocher, S., Fiorelli, L.E., Taborda, J.R.A., and Salgado L., 2020. Two Late Cretaceous sauropods reveal titanosaurian dispersal across South America. Communications Biology 3(1):622. doi: 10.1038/s42003-020-01338-w.

Li, L.G., Li, D.Q., You, H.L., and Dodson, P., 2014. A New Titanosaurian Sauropod from the Hekou Group (Lower Cretaceous) of the Lanzhou-Minhe Basin, Gansu Province, China. PLOS ONE 9 (1): e85979. doi:10.1371/journal.pone.0085979

Mannion, P.D., Upchurch, P., Jin, X., and Zheng, W., 2019. New information on the Cretaceous sauropod dinosaurs of Zhejiang Province, China: impact on Laurasian titanosauriform phylogeny and biogeography. Royal Society Open Science 6(8): 191057. doi:10.1098/rsos.191057

Martínez, R. D. F., M. C. Lamanna, F. E. Novas, R. C. Ridgely, G. A. Casal, J. E. Martínez, J. R. Vita, and L. M. Witmer. 2016. A basal lithostrotian titanosaur (Dinosauria: Sauropoda) with a complete skull: implications for the evolution and paleobiology of Titanosauria. PLoS ONE 11(4):e0151661. doi:10.1371/journal.pone.0151661.

Navarro, B. A. 2019. Postcranial osteology and phylogenetic relationships of the Early Cretaceous titanosaur Tapuiasaurus macedoi Zaher et al. 2011. Master's dissertation. Instituto de Biociências da Universidade de São Paulo, São Paulo, Brazil.

Poropat, S.F., Upchurch, P., Mannion, P.D., Hocknull, S., Kear, B.P., Sloan, T., Sinapius, G.H.K., and Elliott, D.A., 2015. Revision of the sauropod dinosaur Diamantinasaurus matildae Hocknull et al. 2009 from the mid-Cretaceous of Australia: implications for Gondwanan titanosauriform dispersal. Gondwana Research. 27 (3): 995–1033. 

Poropat, S.F., Mannion, P.D., Upchurch, P., Hocknull, S.A., Kear, B.P., Kundrát, M., Tischler, T.R., Sloan, T., Sinapius, G.H.K., Elliott, J.A., and Elliott, D.A., 2016. New Australian sauropods shed light on Cretaceous dinosaur palaeobiogeography. Scientific Reports 6: 34467. doi:10.1038/srep34467

Poropat S. F., Kundrát M., Mannion P. D., Upchurch P., Tischler T. R., and Elliott D. A., 2021. Second specimen of the Late Cretaceous Australian sauropod dinosaur Diamantinasaurus matildae provides new anatomical information on the skull and neck of early titanosaurs. Zoological Journal of the Linnean Society 192 (2): 610–674.

Silva, J.C., Jr., Martinelli, A.G., Iori, F.V., Marinho, T.S., Hechenleitner, E.M., and Langer, M.C., 2021. Reassessment of Aeolosaurus maximus, a titanosaur dinosaur from the Late Cretaceous of Southeastern Brazil. Historical Biology: An International Journal of Paleobiology. in press.  doi:10.1080/08912963.2021.1920016.

Soto, M., Montenegro, F., Mesa, V., and Perea, D., 2022. Sauropod (Dinosauria: Saurischia) remains from the Mercedes and Asencio formations (sensu Bossi, 1966), Upper Cretaceous of Uruguay. Cretaceous Research 131: 105072. doi:10.1016/j.cretres.2021.105072

Wilson, J.A., 2002. Sauropod dinosaur phylogeny: critique and cladistic analysis. Zoological Journal of the Linnean Society 136(2): 215–275.

Wilson, J. A., D. Pol, A. B. Carvalho, and H. Zaher. 2016. The skull of the titanosaur Tapuiasaurus macedoi (Dinosauria: Sauropoda), a basal titanosaur from the Lower Cretaceous of Brazil. Zoological Journal of the Linnean Society 178(3):611–662.

Zaher, H., D. Pol, A. B. Carvalho, P. M. Nascimento, C. Riccomini, P. Larson, R. Juarez-Valieri, R. Pires-Domingues, N. J. da Silva, Jr., and D. de Almeida Campos. 2011. A complete skull of an Early Cretaceous sauropod and the evolution of advanced titanosaurians. PLoS ONE 6(2):e16663. doi:10.1371/journal.pone.0016663.